By the middle of the 20th century, it had begun to seem that biology was almost solved. Charles Darwin’s theory of evolution by natural selection explained how organisms change and adapt. The modern science of genetics showed how it works at the molecular scale. Genes governing the traits of organisms get passed down from parent to offspring, and random mutations create the variations from which natural selection picks the “fittest.” Natural selection and genetics fitted together in what the biologist Julian Huxley christened “the modern synthesis” in his 1942 book. Once it was shown in 1953 that the genes are encoded by DNA, the rest of biology looked like little more than piecing together details.
But not everyone was satisfied. The British biologist Conrad Hal Waddington, known to his friends and colleagues as Wad, thought this focus on genes was all very well. But it wasn’t clear to him, or anyone else, exactly how genes shape the forms and features of organisms — how they reliably generate all the different tissues of the body, in all the right places, during embryonic development. Around the same time that Huxley unveiled the modern synthesis, Waddington presented a novel picture of how this might unfold.
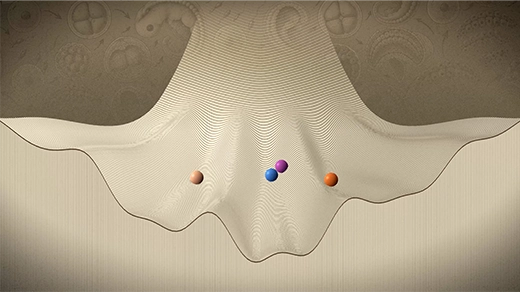
He visualized the developmental process as a landscape with hills and valleys that split every so often like those in a river network. At the very top of the highest hill he imagined a ball, which represented a population of cells in their earliest embryonic form — what we now call stem or pluripotent cells, which have the potential to become any cell type. The progression of the cells towards their fates — to become, say, skin cells, muscle cells, or nerve cells — is like the ball rolling downhill through the landscape.
When the ball reaches a branching point (bifurcation), the model’s “gravity” pulls it to one track or the other: In scientific terms, it must differentiate. Through a particular sequence of such branching decisions, Waddington argued, cells specialize into their mature types, or fates, each expressing a particular set of genes. The cells are restricted to a small number of well-defined states because they are “canalized,” in Waddington’s lexicon: trapped and channeled by the sides of the valley. In this way, a limited number of cell types reliably arise from the activity of an army of genes.
Waddington’s landscape has been “remarkably useful as a conceptual scaffold,” said James Briscoe, a developmental biologist at the Francis Crick Institute in London. “The core ideas — that development is progressive, that cell states are distinct, that bifurcations represent [cell] fate decisions, that canalization implies robustness — all survive.”
“There’s so much richness to some of the concepts Waddington was trying to share,” said Susanne Rafelski, a biochemist at the Institute for Stem Cell and Regenerative Medicine in Seattle.
But the concept was more of a visual metaphor than a representation of an actual biological process. Or so it seemed. In the past several years, researchers have mapped out the real topography of cell-state spaces — in effect, Waddington’s landscapes — from experimental data collected from many thousands of cells over the course of embryonic development. Those analyses are revealing that development is not a mere readout of a genetic program, but rather a dynamic process in which communities of cells build themselves, and the very landscape they navigate, by mutual negotiation and interaction, into an organism.
This cartography of development is now helping researchers understand how identical cells in the early embryo develop into the distinct tissues and cell types of a complex organism. This matters enormously for regenerative medicine and stem-cell engineering, Briscoe said: “If you understand the landscape topology and know where the bifurcations lie, you can in principle design methods that steer cell populations to desired states with precision, rather than by trial and error.”
Waddington’s metaphor, then, could be the key to understanding and reshaping possibilities for what cells, tissues, and embryos can be.
Charting a Landscape
In the 1940s, genetics and embryology were separate sciences; not everyone even believed that genes played a significant role in development. Yet Waddington’s own experiments in embryology, and those of others, convinced him that the formation and patterning of tissues in an embryo were indeed controlled by genes. The cells of different tissues had different groups of genes activated in their chromosomes, he thought. A process of differentiation gradually specialized cells into skin cells, nerve cells, and so on.
Waddington figured that the developmental pathways — for example, the formation of the neural tube from a layer of embryonic tissue called ectoderm, which ultimately develops into the central nervous system — are inevitable once the process has begun, just as water flowing down a river valley is constrained by its surroundings. The path might meander a little, but the valley keeps the river on course. Differentiation corresponds to the branching of a valley, and the final destinations are the mature cell types of the body.
Waddington’s classic drawing of the epigenetic landscape. A ball, representing a pluripotent cell or population, is poised to roll downhill into valleys, each of which represent a specialized cell type, such as a blood cell, liver cell, or brain cell.
From The Strategy of the Genes by C.H. Waddington
Waddington visualized this as a landscape in drawings, but they had “no grounding in physical reality,” wrote Scott Gilbert, a developmental biologist at Swarthmore College in Pennsylvania, in a 1991 essay in Biology & Philosophy. They were useful schematics for thinking about the problem of development, and nothing more.
“Without mathematical content,” Briscoe said, the metaphor “could not distinguish between alternative mechanisms, make quantitative predictions, or be falsified.” As a result, he said, Waddington’s landscape “has sometimes become a cliché rather than a meaningful explanation.”
What, for example, determines the topography of the hills and valleys? In his 1957 book The Strategy of the Genes, Waddington depicted the landscape as he figured it might look from underneath: as a sheet that is tugged into shape by a network of ropes attached to pegs. The pegs represented individual genes, and the ropes their effects on development. Expressing a particular gene — turning it into its corresponding protein — is like pulling on its ropes to change the shape of the sheet.
What determines the landscape’s shape? Waddington sketched a network of pegs and ropes beneath the rolling hills; the pegs are genes, and the ropes are their interconnections. Together they shape the landscape above and represent what we now call gene regulatory networks.
From The Strategy of the Genes by C.H. Waddington
It’s rather more complex than that, Waddington realized, because the ropes are connected in a network. Any one of them might influence the landscape at several points, and any given point on the landscape might be attached to several ropes.
These hidden connections correspond to what researchers now call gene regulatory networks: interactions among genes whereby an increase in the expression of one might change, or regulate, the activity of others. Herein lies the cryptic complexity of development. A given process, such as formation of the neural tube, might be influenced by many interacting genes; there’s no simple relationship between genes (genotype) and the developmental landscape that determines form (phenotype). Gene regulatory networks mediate between them.
It makes no sense, then, to look for genes dedicated to creating specific tissues, organs, or structures in a whole organism, which is one reason Waddington’s metaphor proved useful. The landscape image was “valuable in providing an alternative to a purely gene-centric view of development,” Briscoe said. By emphasizing the landscape’s shape, it pointed “toward system-level properties that cannot be read off from any single gene.”
Gene regulation wasn’t understood when Waddington first devised his landscape and rope network. A few years later, in the early 1960s, it became clear that one gene could turn another on or off. Researchers, such as the complexity theorist Stuart Kauffman, began to construct simple mathematical models of the networks of gene interactions. But too little was then known about real gene networks to connect abstract theory to experiment. “Given that the channels and spheres had no physical reality,” Gilbert wrote, “what was an embryologist supposed to do with them?”
Answers have begun to emerge over the past two decades thanks to new experimental tools for characterizing cell states. Biologists are now finally becoming able to map experimental data to a real mathematical landscape for differentiation and show just how prescient Waddington was.
Fated Attractors
One way to define the state of a given cell in an embryo is by the expression levels of its genes. These levels can now be measured simultaneously in many cells using a technique called single-cell RNA sequencing, which supplies a snapshot of all the different RNA molecules each cell contains. An RNA molecule (or transcript) is a kind of copy of a gene used to translate it into a functional protein, and generally, more RNA transcripts means higher expression of that gene. Each cell type is characterized by particular gene-expression settings, which are inherited when a cell divides. This ensures that a liver cell will stay a liver cell as it progresses through an organism’s development process.
In principle, RNA-sequencing data can be modeled as a high-dimensional mathematical space in which each axis denotes the number of RNA transcripts of a single gene. Such a plot, with maybe thousands of dimensions to represent thousands of genes, is impossible to visualize, but it can be mathematically projected onto a space with fewer dimensions, usually just two, to produce something like the shadow of a complex 3D object.
On such a plot, called a UMAP (uniform manifold approximation and projection), different cell types appear as clusters of points — blood cells cluster together, say, as do cells of the muscle or forebrain — as they share a gene expression profile. Cell lineages follow paths through this map as development proceeds. When the data is mapped through time — in what’s known as a network flow model — it looks very much like a population of cells rolling through a Waddington-like landscape, being channeled along valleys that lead to basins that correspond to distinct cell types.